SLU-PP-332 vs MOTS-c: ERR Agonist vs Mitochondrial Peptide
For laboratory research only. Not for human or animal use. This article gives no dosing, administration or therapeutic advice.
Short answer: SLU-PP-332 and MOTS-c are often grouped together as “exercise mimetics”, but they are different kinds of research tool. SLU-PP-332 is a small synthetic molecule, not a peptide, designed to switch on the estrogen-related receptors ERRα, ERRβ and ERRγ, with its strongest potency at ERRα[1]. MOTS-c is a 16-amino-acid peptide encoded inside the mitochondrial genome; in cells and mice it acts through the folate cycle and AMPK, and under metabolic stress it moves into the nucleus[2][3]. One is a drug-design probe for a nuclear receptor family; the other is a naturally occurring signalling peptide. Almost everything known about both comes from cell cultures and mice.
Why these two get compared
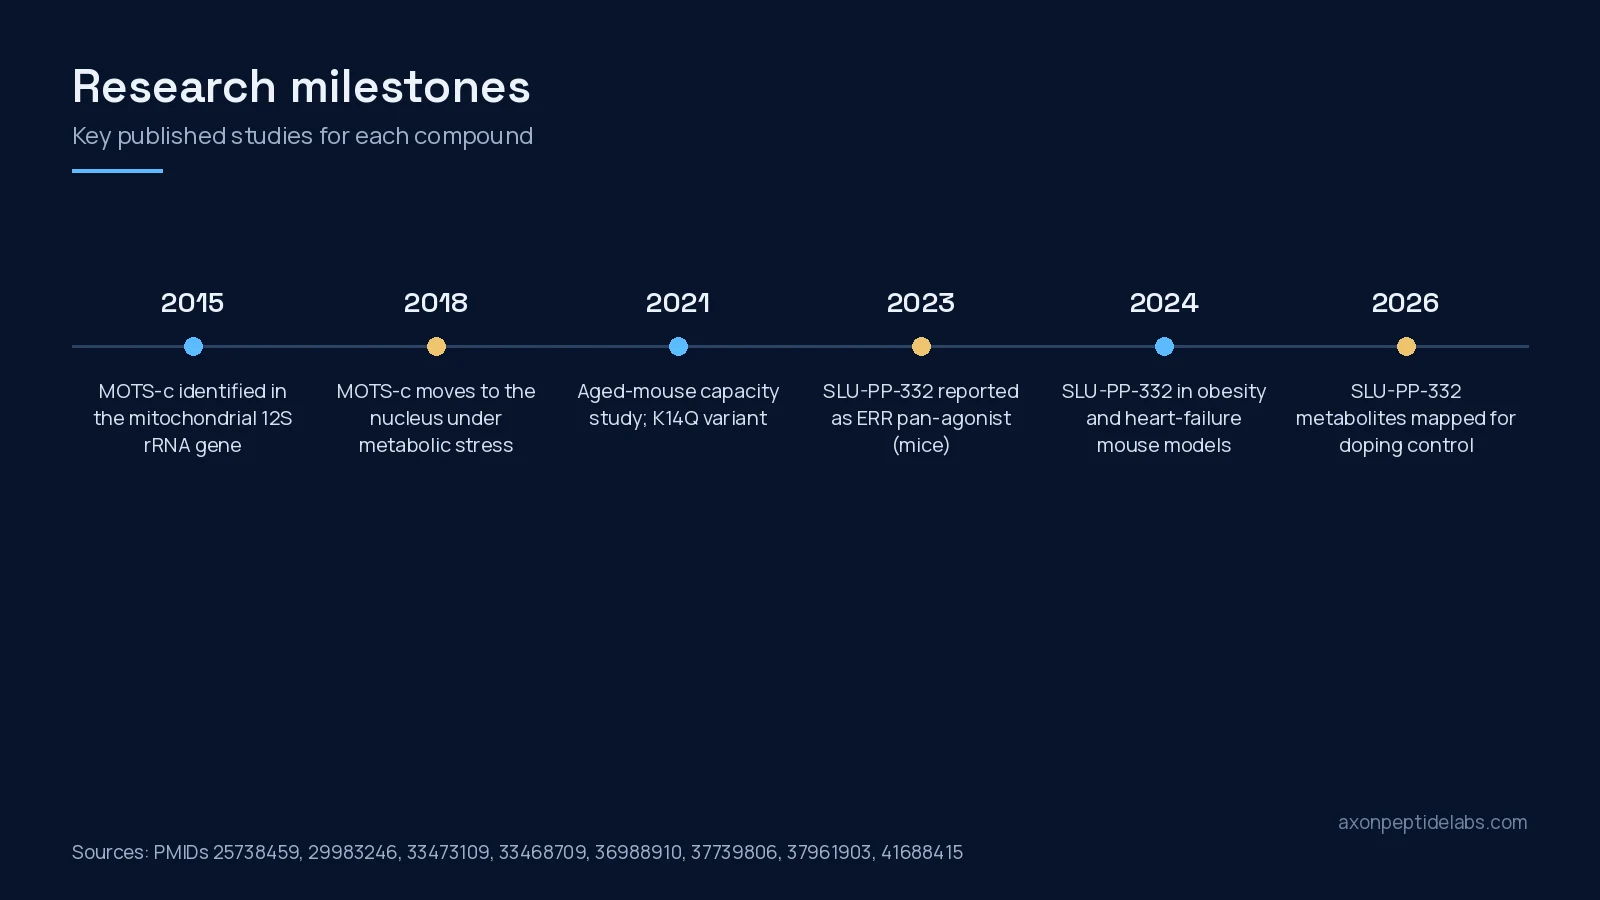
Both compounds sit in the same corner of metabolic research: skeletal muscle, mitochondria and the gene programme that switches on after aerobic exercise. In the 2023 paper that introduced it, SLU-PP-332 raised mitochondrial function and cellular respiration in a skeletal muscle cell line, increased oxidative type IIa fibres in mice and lengthened treadmill endurance, and the endurance effect depended on ERRα[1]. MOTS-c was described in 2015 as a peptide whose main target organ appeared to be skeletal muscle; in mice it prevented diet-induced and age-dependent insulin resistance[2]. A 2021 study then reported that MOTS-c treatment increased physical performance in young, middle-aged and old mice, and that exercise raised endogenous MOTS-c in human muscle and blood[4].
So the overlap is the research question, not the chemistry. The routes in are very different, which is the point of this comparison. For a related metabolic comparison of two non-peptide and peptide tools, see our AOD-9604 vs 5-Amino-1MQ article.
Identity table
Values come from PubChem records, not from certificates of analysis.
| Field | SLU-PP-332 | MOTS-c |
|---|---|---|
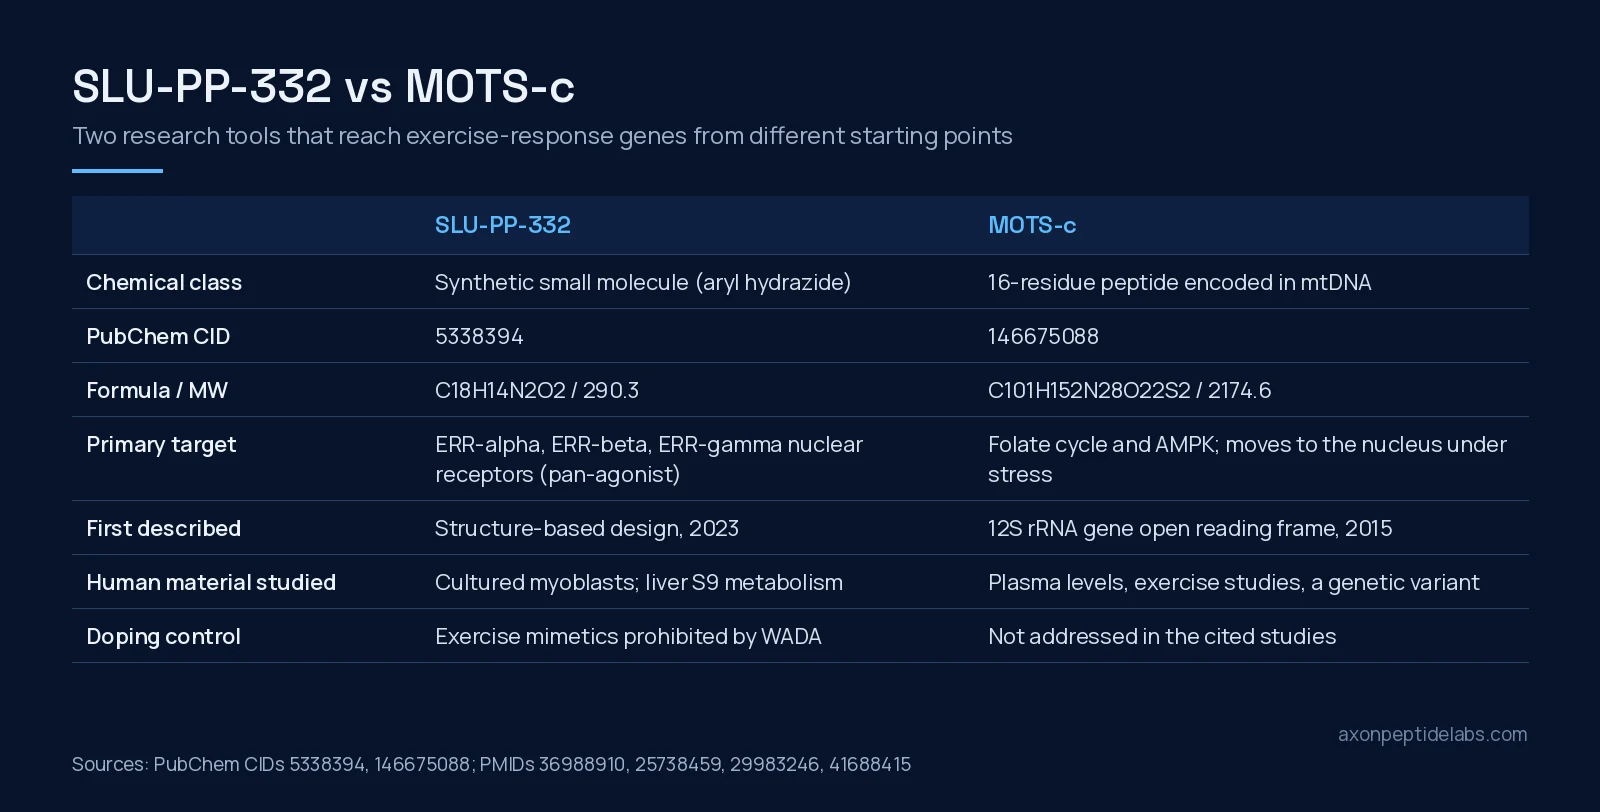
| PubChem CID | 5338394 | 146675088 |
| CAS (PubChem synonyms) | 303760-60-3 | 1627580-64-6 |
| Other names | ERR pan-Agonist 332; 4-hydroxy-N’-(naphthalen-2-ylmethylene)benzohydrazide | Mitochondria-derived peptide MOTS-c; UNII A5CV6JFB78 |
| Molecular formula | C18H14N2O2 | C101H152N28O22S2 |
| Molecular weight | 290.3 g/mol | 2174.6 g/mol |
| Structure | Aryl hydrazide (hydrazone) small molecule; no amino acids | 16 residues, MRWQEMGYIFYPRKLR[2] |
| Where it comes from | Synthetic, structure-based design | Short open reading frame in the mitochondrial 12S rRNA gene |
The molecular weights alone show the gap: MOTS-c is roughly seven times heavier than SLU-PP-332. On an LC-MS trace the two could not be mistaken for each other, and a purity report for one says nothing about the other. Any supplier that lists SLU-PP-332 under “peptides” is using a shop category, not a chemical one.
How SLU-PP-332 works: ERR agonism
The estrogen-related receptors are orphan nuclear receptors. Despite the name they do not bind estrogen; they are transcription factors that control genes for mitochondrial biogenesis, oxidative phosphorylation, fatty acid oxidation and the Krebs cycle[5]. Genetic work had already linked them to muscle exercise capacity, but ERRα agonists had been hard to make and few synthetic agonists worked in vivo[1].
SLU-PP-332 filled that gap as a pan-agonist with enough pharmacokinetic stability to use in mice[1]. Follow-up mouse studies from the same programme reported:
- Diet-induced obese and ob/ob mice: higher energy expenditure and fatty acid oxidation, less fat mass accumulation and better insulin sensitivity[6].
- Pressure-overload heart failure in mice: SLU-PP-332 and a second agonist, SLU-PP-915, improved ejection fraction, reduced fibrosis and increased survival without changing cardiac hypertrophy; ERRγ, not ERRα, was the main mediator in heart tissue[7].
- Aging kidney (21-month-old mice): eight weeks of treatment reversed age-related albuminuria, podocyte loss, mitochondrial dysfunction and inflammatory cytokines, through cGAS-STING and STAT3 signalling[8].
The only human material in the SLU-PP-332 literature we found is cells. Myoblasts taken during hip surgery from physically inactive women were treated with SLU-PP-332 in culture; ERRα, PGC-1α and SIRT1 went up, NOX4 went down, oxidative stress and senescence markers fell and myotube formation increased[9]. That is a cell-culture result, and the study had 20 participants in total.
How MOTS-c works: a peptide from the mitochondrial genome
MOTS-c stands for mitochondrial open reading frame of the 12S rRNA type-c. Its discovery paper reported that it inhibits the folate cycle and the de novo purine synthesis tied to it, which leads to AMPK activation[2]. Three years later the same field showed that MOTS-c is not only a cytoplasmic signal: after glucose restriction it translocated to the nucleus in an AMPK-dependent way and regulated nuclear genes, including antioxidant response element genes, while interacting with NRF2[3].
In muscle models, MOTS-c prevented palmitic-acid-induced atrophy in C2C12 myotubes and lowered plasma myostatin in diet-induced obese mice, working through AKT and FOXO1[10]. In rats and mice, weeks of voluntary running raised MOTS-c protein in several muscles, and a single administration to untrained mice increased running time and distance in an acute test[11]. Note the direction in that last study: training raised MOTS-c, and MOTS-c changed an acute run. It is not evidence that MOTS-c replaces training.
Side-by-side comparison
| Aspect | SLU-PP-332 | MOTS-c |
|---|---|---|
| What it is | Synthetic ERRα/β/γ pan-agonist[1] | Mitochondrial-derived peptide, 16 residues[2] |
| Main mechanism reported | Direct activation of nuclear receptors that drive an aerobic exercise gene programme[1] | Folate cycle inhibition and AMPK activation; nuclear translocation under stress[2][3] |
| Muscle findings | More type IIa oxidative fibres and longer endurance in mice[1] | Better physical performance in young, middle-aged and old mice[4] |
| Metabolic models | Diet-induced obese and ob/ob mice[6] | High-fat-fed and aged mice[2] |
| Other organs studied | Heart (pressure overload), aging kidney[7][8] | Skeletal muscle atrophy signalling[10] |
| Human data | Cultured myoblasts only[9] | Endogenous plasma and muscle levels; genetic variant studies[12][13] |
| Known limitation | Described by its developers as lacking oral bioavailability[5] | An East Asian mtDNA variant (K14Q) lowers its activity[13][14] |
What human studies actually measured
This is where the two diverge most, and where many online comparisons blur things. For MOTS-c, human studies measure the body’s own peptide. Plasma MOTS-c was similar in lean and obese adults; it correlated with insulin-sensitivity indexes overall, but when the groups were analysed separately the association held only in lean individuals[12]. In a randomised exercise trial in breast cancer survivors, 16 weeks of aerobic and resistance training raised plasma MOTS-c in non-Hispanic White participants but not in Hispanic participants[15]. A meta-analysis of three Japanese and multi-ethnic cohorts linked the K14Q variant to type 2 diabetes prevalence in men, and K14Q-MOTS-c lost the effects of normal MOTS-c in male mice[13]. In Japanese athletes, carriers of the same variant had more fast-twitch fibre markers[14].
None of these studies gave people MOTS-c. They are observational or genetic, and they show associations that differ by sex, ethnicity and body composition. For SLU-PP-332 there are no human studies of any kind beyond cultured cells and liver fractions.
The doping-control angle
SLU-PP-332 has reached the anti-doping literature before it has reached a clinical trial. A 2026 study notes that the World Anti-Doping Agency prohibits exercise mimetics and metabolic modulators in sport, and maps 22 in vitro metabolites of SLU-PP-332 made by human liver S9 fractions, with several flagged as markers for doping tests[16]. A second group characterised SLU-PP-332 and SLU-PP-915 by high-resolution mass spectrometry, found nine metabolites for SLU-PP-332 including Phase II conjugates, and framed the work around detecting misuse[17]. For a lab, the useful side of this work is analytical: published LC-HRMS data now exist for identity checks.
Chemists are also still working out the scaffold. A 2026 structure-activity study described SLU-PP-332 as a widely used benchmark probe, but found analogues with comparable ERR responses and better ligand efficiency, solubility or metabolic stability[18]. The same programme has reported SLU-PP-915, a chemically distinct, orally bioavailable ERR agonist, because SLU-PP-332 lacks oral bioavailability[5].
What the evidence does not show
- No head-to-head study. We found no paper that tests SLU-PP-332 against MOTS-c in the same model. Any ranking of one over the other is speculation.
- No human interventional data for either. Neither compound has a published trial in which people received it. Mouse endurance, fat-mass and insulin-sensitivity findings do not establish any effect in humans.
- One main source for SLU-PP-332. Most in vivo SLU-PP-332 data come from a single drug-discovery programme[1][6][7]. Independent replication in other labs is still limited.
- Mixed human associations for MOTS-c. Circulating levels did not differ between lean and obese adults, and exercise raised them in one ethnic group but not another in the same trial.
- Long-term safety is unstudied. The cited papers report short animal studies; none establishes long-term safety in any species.
Documentation for our listings
Our COA page lists MOTS-C 10mg (pen), batch MP-MOTS-10-041626, purity 99.89%, dated 28 APR 2026, lab testides.com. That report covers the batch it names; check the batch on the label of the item you receive against it. No certificate is posted for SLU-PP-332 on our COA page at the time of writing. SLU-PP-332 is listed as SLU-PP-332 capsules; MOTS-c is available as MOTS-C 10 mg and in pen format. Background on the peptide and its documentation is on our MOTS-c Canada page. Researchers comparing suppliers can buy lab-tested peptides in Canada through our main catalogue.
Frequently asked questions
Is SLU-PP-332 a peptide?
No. PubChem records SLU-PP-332 as a small molecule with the formula C18H14N2O2 and a molecular weight of 290.3, an aryl hydrazide with no amino acids. It is often sold beside peptides, but chemically it is a synthetic ERR agonist designed by structure-based drug design.
How does MOTS-c differ from SLU-PP-332 in mechanism?
MOTS-c is a 16-residue peptide encoded in mitochondrial DNA that inhibits the folate cycle, activates AMPK and can move to the nucleus under metabolic stress. SLU-PP-332 binds and activates the estrogen-related receptors ERR-alpha, beta and gamma directly, switching on an aerobic exercise gene programme in mouse muscle.
Have SLU-PP-332 or MOTS-c been tested in human trials?
Not as administered compounds in the studies we cite. SLU-PP-332 human data are limited to cultured myoblasts and liver fractions. Human MOTS-c studies measure the body’s own peptide in plasma or muscle, or look at a genetic variant; none gave participants MOTS-c.
Has anyone compared SLU-PP-332 and MOTS-c directly?
We found no published head-to-head study. Their evidence comes from different labs, models and endpoints, so direct claims about which is stronger are not supported by the literature.
Why does SLU-PP-332 appear in anti-doping research?
The World Anti-Doping Agency prohibits exercise mimetics and metabolic modulators in sport. Two 2026 studies used human liver fractions and high-resolution mass spectrometry to map SLU-PP-332 metabolites so testing labs can detect misuse.
Does Axon Peptide Labs post a COA for these products?
Our COA page lists MOTS-C 10mg (pen), batch MP-MOTS-10-041626, 99.89% purity, dated 28 APR 2026, tested by testides.com. No certificate is posted for SLU-PP-332 on our COA page at the time of writing.
References
- Billon C, Sitaula S, Banerjee S et al. (2023). Synthetic ERRα/β/γ Agonist Induces an ERRα-Dependent Acute Aerobic Exercise Response and Enhances Exercise Capacity. ACS Chem Biol. PMID: 36988910. doi: 10.1021/acschembio.2c00720.
- Lee C, Zeng J, Drew BG et al. (2015). The mitochondrial-derived peptide MOTS-c promotes metabolic homeostasis and reduces obesity and insulin resistance. Cell Metab. PMID: 25738459. doi: 10.1016/j.cmet.2015.02.009.
- Kim KH, Son JM, Benayoun BA et al. (2018). The Mitochondrial-Encoded Peptide MOTS-c Translocates to the Nucleus to Regulate Nuclear Gene Expression in Response to Metabolic Stress. Cell Metab. PMID: 29983246. doi: 10.1016/j.cmet.2018.06.008.
- Reynolds JC, Lai RW, Woodhead JST et al. (2021). MOTS-c is an exercise-induced mitochondrial-encoded regulator of age-dependent physical decline and muscle homeostasis. Nat Commun. PMID: 33473109. doi: 10.1038/s41467-020-20790-0.
- Billon C, Appourchaux K, Côté I et al. (2026). An orally active estrogen receptor-related receptor agonist, SLU-PP-915, enhances aerobic exercise capacity. J Pharmacol Exp Ther. PMID: 41421047. doi: 10.1016/j.jpet.2025.103787.
- Billon C, Schoepke E, Avdagic A et al. (2024). A Synthetic ERR Agonist Alleviates Metabolic Syndrome. J Pharmacol Exp Ther. PMID: 37739806. doi: 10.1124/jpet.123.001733.
- Xu W, Billon C, Li H et al. (2024). Novel Pan-ERR Agonists Ameliorate Heart Failure Through Enhancing Cardiac Fatty Acid Metabolism and Mitochondrial Function. Circulation. PMID: 37961903. doi: 10.1161/CIRCULATIONAHA.123.066542.
- Wang XX, Myakala K, Libby AE et al. (2023). Estrogen-Related Receptor Agonism Reverses Mitochondrial Dysfunction and Inflammation in the Aging Kidney. Am J Pathol. PMID: 37717940. doi: 10.1016/j.ajpath.2023.07.008.
- Bonanni R, Falvino A, Matticari A et al. (2025). Targeting ERRs to counteract age-related muscle atrophy associated with physical inactivity: a pilot study. Front Physiol. PMID: 40692696. doi: 10.3389/fphys.2025.1616693.
- Kumagai H, Coelho AR, Wan J et al. (2021). MOTS-c reduces myostatin and muscle atrophy signaling. Am J Physiol Endocrinol Metab. PMID: 33554779. doi: 10.1152/ajpendo.00275.2020.
- Hyatt JK (2022). MOTS-c increases in skeletal muscle following long-term physical activity and improves acute exercise performance after a single dose. Physiol Rep. PMID: 35808870. doi: 10.14814/phy2.15377.
- Cataldo LR, Fernández-Verdejo R, Santos JL et al. (2018). Plasma MOTS-c levels are associated with insulin sensitivity in lean but not in obese individuals. J Investig Med. PMID: 29593067. doi: 10.1136/jim-2017-000681.
- Zempo H, Kim SJ, Fuku N et al. (2021). A pro-diabetogenic mtDNA polymorphism in the mitochondrial-derived peptide, MOTS-c. Aging (Albany NY). PMID: 33468709. doi: 10.18632/aging.202529.
- Kumagai H, Natsume T, Kim SJ et al. (2022). The MOTS-c K14Q polymorphism in the mtDNA is associated with muscle fiber composition and muscular performance. Biochim Biophys Acta Gen Subj. PMID: 34728329. doi: 10.1016/j.bbagen.2021.130048.
- Dieli-Conwright CM, Sami N, Norris MK et al. (2021). Effect of aerobic and resistance exercise on the mitochondrial peptide MOTS-c in Hispanic and Non-Hispanic White breast cancer survivors. Sci Rep. PMID: 34413391. doi: 10.1038/s41598-021-96419-z.
- Avliyakulov NK, Sobolevsky T, Ahrens E (2026). Analysis and Identification of In Vitro Metabolites of Exercise Mimetic SLU-PP-332 ERRα/β/γ Agonist for Doping-Control Purposes. Drug Test Anal. PMID: 41688415. doi: 10.1002/dta.70035.
- Möller T, Krug O, Thevis M (2026). In Vitro Metabolism and Analytical Characterization of SLU-PP-332 and SLU-PP-915: Novel Pan-ERR Agonists With Doping Potential. Rapid Commun Mass Spectrom. PMID: 41588687. doi: 10.1002/rcm.70039.
- Okda HE, Zhao P, Hayes M et al. (2026). Chemical optimization of the exercise mimetic SLU-PP-332 enables insight into estrogen-related receptor signaling. Int J Biol Macromol. PMID: 41850449. doi: 10.1016/j.ijbiomac.2026.151450.